
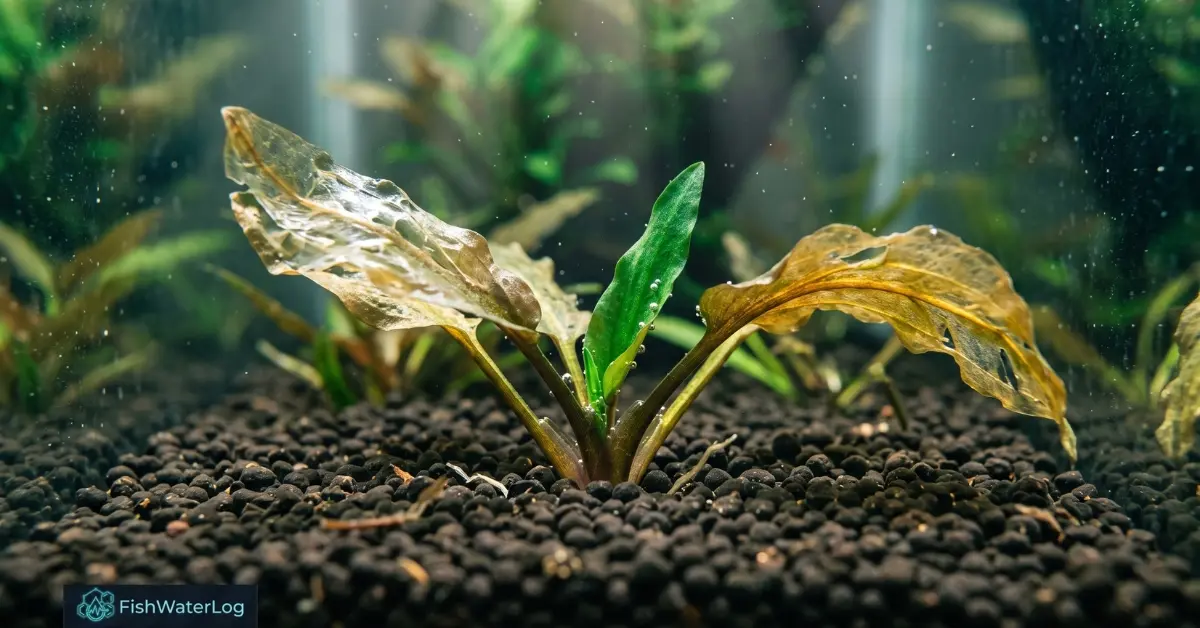
Introducing fresh botanical specimens into a newly scaped tank represents a foundational milestone in aquatic husbandry, yet the rapid deterioration of vibrant foliage into translucent, gelatinous detritus within 48 to 96 hours frequently alarms practitioners. When observing sudden foliar collapse, aquarists invariably ask why are new aquarium plants melting and dying despite careful planting, high-grade aquasoil, and balanced water columns. In the vast majority of cases, acute leaf dissolution does not signify terminal botanical mortality. Instead, this initial breakdown reflects an aggressive, metabolically driven morphological remodeling process as amphibious macrophytes undergo an emersed to submerged transition from commercial greenhouse cultivation to a fully aquatic environment.
Executing a reliable aquarium plant melt recovery requires distinguishing between adaptive cellular senescence and lethal meristematic rot. While surface-level hobbyist guides advise passively waiting out the decay, unaddressed secondary biochemical stressors—such as surges in labile dissolved organic carbon, acute osmotic shock in planted tanks, and localized rhizosphere hypoxia—can quickly transform a natural physiological shift into an ecosystem-wide crisis. By aligning cellular plant biology with disciplined nutrient delivery, photoperiod moderation, and active waste export, aquarists can arrest tissue necrosis and accelerate the emergence of healthy, submersed-adapted growth.
Table of Contents
Competitor Landscape Audit and Unaddressed Botanical Content Gaps
A rigorous audit of mainstream planted aquarium literature reveals that most hobbyist resources treat foliar decay with superficial, observational advice. Standard guides routinely reassure keepers that melting plants will regrow on their own, advising patience or basic trimming without addressing the underlying biochemical catalysts.
Navigating an efficient aquarium plant melt recovery requires closing the technical data gaps left open by mainstream publications:
- Enzymatic Lag Phases: Mainstream guides rarely explain that transitioning plants face a multi-day delay while synthesizing carbonic anhydrase, leaving them vulnerable to severe carbon starvation in the presence of intense lighting.
- Substrate Dynamics and Redox Collapse: Conventional articles warn hobbyists not to uproot plants, but they fail to detail how stagnant interstitial pore water induces rhizosphere hypoxia, turning benign leaf shed into irreversible anaerobic crown necrosis.
- Osmoregulatory Mechanics: Standard blogs overlook how uncompensated evaporative mineral shifts and tap-water top-offs cause osmotic shock in planted tanks, bursting delicate vacuolar membranes in newly forming submerged leaves.
- Heterotrophic Carbon Surges: Most platforms ignore the spike in Labile Dissolved Organic Carbon (LDOC) caused by melting leaves, which drives the water column’s Carbon-to-Nitrogen (C:N) ratio out of balance and fuels cloudy bacterial blooms.
Why Are New Aquarium Plants Melting and Dying? Primary Physiological Triggers
To identify the root cause of foliar loss and prevent complete botanical collapse, aquarists must understand why are new aquarium plants melting and dying through four distinct physiological and environmental triggers.
Emersed-to-Submerged Morphological Reconfiguration
Over 85% of commercial aquatic flora—including common Cryptocoryne, Echinodorus, and stem plants—are cultivated in commercial nurseries under emersed, greenhouse conditions. Aerial leaves develop thick, waxy aerial cuticles to prevent desiccation, heavy lignin-reinforced cell walls to remain upright, and open stomata for direct atmospheric carbon absorption.
When placed underwater, this terrestrial structure becomes a liability. Gas diffusion in water is nearly 10,000 times slower than in air. The waxy cuticle blocks dissolved gases and nutrients from passing through the leaf surface, while aerial stomata cease to function. Unable to alter mature leaves, the plant undergoes an emersed to submerged transition, actively dismantling obsolete foliage so the central meristem can redirect resources toward building thin, cuticle-free aquatic leaves designed for direct dissolved nutrient uptake.
Osmotic Pressure Gradients, TDS Creep, and Chemical Shock
Sharp water chemistry differences between nursery production tanks and domestic aquaria trigger rapid osmotic shock in planted tanks. Plant cell walls rely on steady internal turgor pressure. Plunging a specimen grown in soft water into hard, high-TDS domestic conditions pulls water rapidly out of the central vacuoles via plasmolysis, causing cellular membranes to collapse. Stabilizing pure water source parameters and preventing TDS creep in aquarium RO/DI systems protects newly submerged tissues from sudden osmoregulatory collapse.
Mechanical Root Hair Trauma and Rhizosphere Disruption
Heavy root-feeding flora rely on delicate, single-celled root hairs to absorb trace minerals and macronutrients. Transport, rockwool extraction, and planting with hard aquascaping tweezers shear away these fragile root structures. Stripped of both foliar absorption and functional root uptake, the plant enters an acute water and nutrient deficit, shedding older external foliage to preserve internal reserves for subterranean root regeneration.
Photoperiod Mismatch and Photosynthetic Lag
Exposing freshly planted botanicals to extended periods of intense LED light triggers a severe photoperiod acclimation mismatch. During the initial transition phase, plants have not yet established their underwater light-harvesting enzymes. When inundated with high-energy photons they cannot process, excess light energy generates damaging reactive oxygen species (ROS) that bleach cellular chloroplasts and dissolve leaf blades. Establishing a balanced aquarium lighting photoperiod prevents photo-oxidative stress while carbon-fixation enzymes adjust.
Advanced Biogeochemical Mechanisms Overlooked by Standard Guides
Understanding why are new aquarium plants melting and dying requires looking beneath superficial leaf discoloration and examining the underlying biophysical chemistry of closed aquatic ecosystems. Standard hobbyist advice frequently misinterprets foliar collapse as passive rot, leading to improper maintenance interventions that derail aquarium plant melt recovery. A successful transition relies on understanding five interconnected biochemical mechanisms that dictate whether an aquatic macrophyte regenerates or undergoes irreversible crown necrosis.
Cellular Autophagy and Macronutrient Resorption Kinetics
Plant melt is not passive environmental rot; it is a tightly regulated, genetically programmed process of cellular autophagy and internal nutrient translocation. Before an aquatic plant severs an aerial leaf at its basal abscission zone during the emersed to submerged transition, specialized proteolytic and nucleolytic enzymes dismantle internal chloroplasts, nucleic acids, and structural phospholipids within the senescing blade.
Through this autophagic pathway, the macrophyte actively mobilizes and resorbs mobile macronutrients—predominantly nitrogen (N), phosphorus (P), potassium (K), and magnesium (Mg)—alongside non-structural carbohydrates, pumping them down the petiole into the basal crown, rhizome, or root stock. This internal salvage operation fuels the initial generation of submerged-adapted foliage.
Consequently, pruning yellowing leaves prematurely starves the specimen of critical energy reserves. Aquarists should only excise foliage once the leaf lamina turns glassy, limp, and structurally translucent, signaling that cellular nutrient resorption is complete and physical cellular lysis has begun. For empirical research on terrestrial leaf stress and morphological acclimation during submergence in aquarium flora, consult the botanical study on Hygrophila difformis hosted by the National Center for Biotechnology Information (NCBI).
Labile Dissolved Organic Carbon (LDOC) Surges and Heterotrophic Blooms
Once cellular lysis occurs, decaying emersed foliage leaches substantial concentrations of Labile Dissolved Organic Carbon (LDOC)—such as simple carbohydrates, low-molecular-weight exudates, and free amino acids—directly into the water column. In a balanced, oligotrophic aquarium, the Carbon-to-Nitrogen (C:N) ratio remains stabilized below 5:1, enabling autotrophic nitrifying biofilms to maintain biological equilibrium.
A sudden spike in decomposing biomass pushes the C:N ratio well above 5:1, triggering competitive exclusion. Fast-growing heterotrophic bacteria reproduce via binary fission every 15 to 20 minutes, yielding 0.35 to 0.45 mg of dry cell mass per milligram of organic waste metabolized. In comparison, autotrophic nitrifiers require 12 to 36 hours to double, yielding only 0.05 to 0.10 mg of biomass. This explosive heterotrophic surge consumes substantial dissolved oxygen and requires immediate intervention for clearing aquarium water cloudy white from bacterial blooms before developing crowns suffocate.
Ammonia Equilibrium Shifts and Nitrifier Suppression
As heterotrophic populations decompose structural plant proteins, they mineralize organic nitrogen into Total Ammonia Nitrogen (TAN), which exists in dynamic equilibrium between ionized ammonium (NH4+) and toxic un-ionized ammonia (NH3):
NH3(g) + nH2O(l) ⇌ NH3·nH2O(aq) ⇌ NH4+ + OH– + (n-1)H2O(l)
Un-ionized ammonia (NH3) is a lipid-soluble, uncharged molecule that freely diffuses across biological membranes, generating severe oxidative stress within developing botanical meristems and fish gill lamellae alike. Simultaneously, the heavy biological oxygen demand (BOD) exerted by heterotrophs can drive dissolved oxygen (DO) downward toward critical 2.0 mg/L thresholds. Maintaining an established aquarium nitrogen cycle and biofiltration network dominated by Nitrospira biofilms ensures ammonia spikes are oxidized before free NH3 triggers staghorn or black beard algae on stressed foliage.
The Carbon-Fixation Lag Phase and Biogenic Decalcification Trap
Aerial foliage relies on open atmospheric stomata to absorb gaseous carbon dioxide. When submerged, plants must overhaul their photosynthetic machinery by synthesizing aqueous transport enzymes—most notably carbonic anhydrase—to pull dissolved inorganic carbon across liquid boundary layers. This carbon-fixation lag phase typically persists for 7 to 14 days, during which the plant’s Calvin cycle operates at reduced metabolic efficiency.
If intense lighting is maintained in systems lacking supplemental CO2, carbon-starved plants attempt to extract inorganic carbon directly from dissolved bicarbonate ions (HCO3–) through biogenic decalcification:
Ca2+ + 2HCO3– → CO2 + H2O + CaCO3↓
Splitting bicarbonates consumes nearly twice the cellular ATP of free CO2 assimilation and depletes carbonate hardness (KH) below the vital 50 mg/L (CaCO3) safety buffer. Furthermore, this reaction precipitates an abrasive, alkaline white crust of insoluble calcium carbonate (CaCO3) directly across leaf surfaces, physically blocking light transmission and exhausting the plant’s remaining carbohydrate reserves. Understanding the dynamics of biogenic decalcification and KH loss is vital to prevent severe carbonate exhaustion during early plant establishment.
Rhizosphere Hypoxia and Anaerobic Crown Necrosis
In mature, established aquatic flora, photosynthetic oxygen generated in the foliage travels downward through internal aerenchyma channels and diffuses out of root tips—a process known as radial oxygen loss (ROL) that maintains an oxygenated rhizosphere. When extensive foliar collapse occurs, such as during classic Cryptocoryne melt, internal oxygen transport ceases completely.
In fine, compacted, or detritus-laden substrates lacking pore-water circulation, interstitial dissolved oxygen rapidly drops to zero, inducing acute rhizosphere hypoxia. Under these reducing conditions, anaerobic sulfate-reducing bacteria produce phytotoxic hydrogen sulfide (H2S). This toxic compound attacks the dormant root base, converting a manageable leaf adaptation phase into fatal anaerobic crown rot.
Step-by-Step Aquarium Plant Melt Recovery Protocol (Core Action Checklist)
Executing an effective aquarium plant melt recovery requires a structured intervention that supports internal nutrient reallocation while keeping the surrounding water column chemically pristine. Rather than wondering helplessly why are new aquarium plants melting and dying, aquarists must address the underlying physiological shifts through disciplined, proactive maintenance.
To successfully halt tissue decay and stabilize water parameters during an active melt event, implement the following core action checklist:
- Retain Chlorotic Foliage Until Resorption Completes: Allow pale or yellowing outer leaves to remain attached temporarily so the plant can translocate mobile nitrogen, phosphorus, and potassium into the central crown.
- Prune Translucent and Lysed Tissue at the Petiole Base: Snip away leaves that have turned brown, glassy, or gelatinous using sharp aquascaping shears, and siphon out detached debris immediately to prevent surges in organic carbon.
- Leave Subterranean Roots Completely Undisturbed: Never uproot or reposition a melting specimen; disturbing the substrate shears off microscopic root hairs and resets the plant’s hormonal acclimation timeline.
- Insert Basal Root Fertilizers Near Heavy Feeders: Place nutrient-rich root tabs 2 to 3 cm from the base of Cryptocoryne and Echinodorus specimens to provide developing roots with direct access to minerals.
- Reduce Photoperiod to 6 Hours Daily: Down-regulate LED lighting duration to 6 hours per day at moderate intensity during the 14-day enzyme lag phase to eliminate photo-oxidative stress and suppress opportunistic algae.
- Perform 30% to 50% Weekly Water Exchanges: Conduct temperature-matched partial water changes to export leached ammonia and maintain a stable carbonate hardness buffer above 50 mg/L.
Phase 1: Selective Necrotic Pruning Versus Premature Defoliation
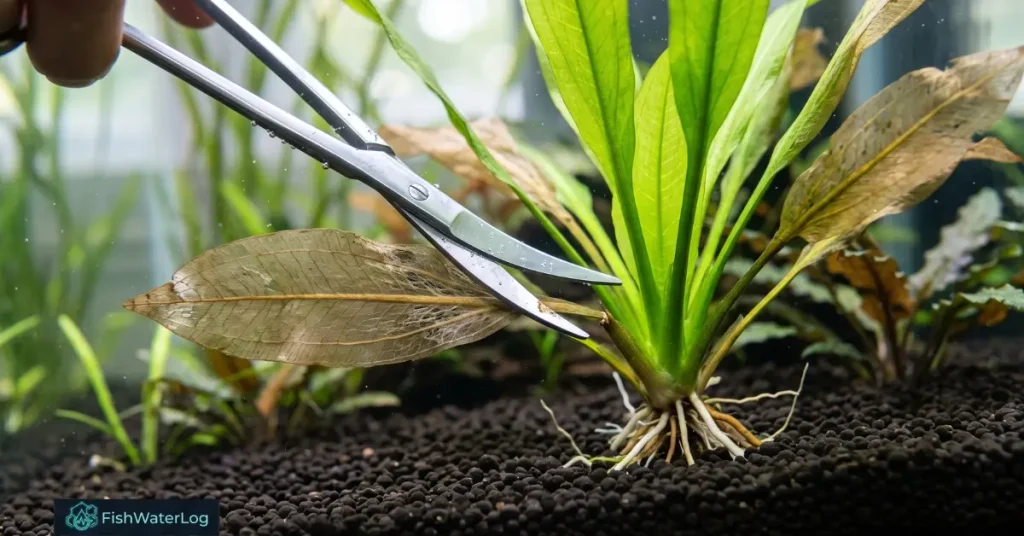
Phase 1 of aquarium plant melt recovery: selectively snipping lysed, glassy outer foliage at the petiole base without disturbing the active crown or subterranean roots.During the initial stages of the emersed to submerged transition, distinguishing between active nutrient resorption and actual necrotic decay is critical. Leaves that are pale, light green, or yellowing along the outer margins are actively exporting vital amino acids and mobile minerals to the meristem; cutting them prematurely halts cellular autophagy and starves the plant.
Excise foliage only after the leaf lamina turns brown, glassy, limp, or slimy. At this stage, cell walls have ruptured, resorption has ceased, and the rotting tissue will rapidly leach organic waste into the water. Using curved stainless-steel aquascaping shears, cut the decaying petiole cleanly near the base without nicking the central crown or rhizome. Siphon out detached debris immediately to prevent heterotrophic bacterial blooms and localized ammonia spikes.
Phase 2: Root Zone Preservation and Basal Mineral Delivery
Preserving the physical architecture of the root zone is the single most decisive factor in achieving complete aquarium plant melt recovery. Pulling a melting plant out of the substrate to inspect its root system shears off fragile, single-celled root hairs and forces the specimen to restart root regeneration from zero.
Instead, evaluate crown and rhizome viability in situ by gently brushing away a few granules of substrate at the base. As long as the crown or rhizome feels firm to the touch and displays white, tan, or healthy green tissue, the plant possesses the energy reserves needed to produce new aquatic shoots. Conversely, if an epiphytic Anubias or Bucephalandra rhizome turns black, mushy, and foul-smelling, excise the rotted portion using a sterile blade at least 5 mm into healthy green tissue. Because defoliated plants temporarily lack functional leaves for water-column nutrient uptake, insert root tabs near the root zone or learn how to recharge old aquarium soil so regenerating root hairs have immediate access to bioavailable iron, potassium, and phosphorus.
Phase 3: Photoperiod Down-Regulation and Spectral Management
While transitioning plants synthesize carbonic anhydrase and adapt to aqueous gas diffusion over the initial 7-to-14-day lag phase, restrict overhead LED fixtures to a 6-hour daily photoperiod at 50% to 60% intensity. Moderating the Daily Light Integral (DLI) provides essential photoperiod acclimation, preventing excess photon inundation that produces destructive reactive oxygen species (ROS) in transitioning foliage.
In aquariums equipped with non-dimmable, fixed-intensity lights, introducing hardy floating plants for aquarium aeration such as Limnobium laevigatum (Amazon Frogbit) or Phyllanthus fluitans (Red Root Floater) across 30% to 50% of the water surface naturally diffuses harsh lighting while hyper-accumulating excess ammonium and nitrates leached by melting submerged stems.
Phase 4: Osmotic Stabilization and Organic Waste Export
Consistent 30% to 50% weekly water changes dilute dissolved organic carbon, purge un-ionized ammonia, and restore essential carbonate buffers. When acclimating species prone to rapid breakdown, such as during severe Cryptocoryne melt, maintaining water-column macronutrients according to modified Redfield stoichiometry—targeting Nitrate (NO3–) at 10–20 ppm and Phosphate (PO43-) at 1.0–2.0 ppm—prevents nutrient starvation once new submerged shoots emerge.
Avoid dosing glutaraldehyde-based “liquid carbon” supplements onto actively melting plants. Glutaraldehyde acts as a potent cellular cross-linking agent and algaecide that induces severe epidermal necrosis and vacuolar collapse in delicate transitioning foliage, particularly in sensitive genera such as Vallisneria and Cryptocoryne. Maintain stable osmotic conditions with zero-TDS top-offs to prevent osmotic shock while new foliage establishes.
Comparative Matrix: Plant Melt Triggers, Diagnostic Symptoms, and Recovery Actions
Diagnosing why are new aquarium plants melting and dying requires differentiating normal morphological acclimation from fatal parameter crashes. Implementing a targeted aquarium plant melt recovery relies on identifying the exact biochemical catalyst behind foliar breakdown before intervening.
| Primary Trigger | Visual Diagnostic Symptoms | Biochemical Mechanism | Targeted Recovery Action | Expected Rebound |
|---|---|---|---|---|
🌱
Emersed-to-Submerged Transition
Adaptive Senescence | Outer rigid leaves turn yellow, then translucent from margins inward; central crown remains firm. | Cellular autophagy resorbs NPK from thick-cuticle aerial leaves to build thin aquatic foliage. | Leave roots undisturbed; prune only fully translucent leaves; maintain a 6-hour photoperiod. | 14–28 Days Standard cycle |
⚡
Acute Osmotic / TDS Shock
Membrane Plasmolysis | Rapid, tank-wide wilting and glassy disintegration of all leaves within 24 to 48 hours of planting. | Abrupt GH/KH/TDS shifts collapse vacuolar turgor pressure and rupture delicate cellular membranes. | Stabilize top-offs with 0-TDS RO/DI water; drip-acclimate new specimens over 30 to 45 minutes. | 7–21 Days Rapid recovery |
🧪
Carbon-Fixation Lag & Decalcification
Enzymatic Deficit | Gritty white CaCO3 crust on upper leaf surfaces; brittle, disintegrating leaf blades; dropping KH. | High lighting without free CO2 forces plants to strip carbon from HCO3–, exhausting cellular ATP. | Inject pressurized CO2 (15–25 mg/L) or dim lighting; maintain carbonate hardness above 50 mg/L (4 dKH). | 14–35 Days Enzyme adaptation |
🍂
Nutrient Starvation (NPK / Iron)
Substrate Exhaustion | Older lower leaves yellow uniformly (Nitrogen) or develop necrotic pinholes (Potassium) before melting. | Lack of basal or water-column minerals forces internal cannibalization of lower structural leaves. | Insert substrate root tabs near heavy feeders; maintain NO3– at 10–20 ppm and PO43- at 1–2 ppm. | 14–35 Days Fertilization lag |
🧫
Tissue Culture Agar Toxicity
Heterotrophic Rot | Basal stems turn brown and mushy from the substrate line upward; white fungal fuzz (Saprolegnia) at plant base. | Residual sugar-rich tissue culture gel fuels anaerobic bacteria and localized NH3 toxicity at the root collar. | Rinse tissue culture clumps thoroughly in lukewarm water prior to planting; execute a 50% water change. | 10–21 Days Post-rinse stabilization |
⚠️
Anaerobic Rhizome / Crown Rot
Rhizosphere Hypoxia | Rhizome or crown turns black, mushy, and foul-smelling; healthy green leaves detach cleanly at the base. | Buried epiphytic rhizomes or hypoxic substrate pockets suffocate meristematic tissue and generate H2S. | Unbury epiphytes immediately; excise black necrotic tissue with a sterile blade 5 mm into healthy green tissue. | 21–42+ Days Slow meristem rebirth |
Species-Specific Melt Profiles and Regeneration Timelines
Aquatic macrophytes do not respond uniformly during an active melt event. Distinct vascular anatomies, root storage capacities, and metabolic growth rates dictate the trajectory of aquarium plant melt recovery across different botanical families.
Cryptocoryne Species (The Classic “Crypt Melt” Phenomenon)
Members of the genus Cryptocoryne (including C. wendtii, C. parva, C. lutea, and C. balansae) exhibit extreme physiological sensitivity to environmental shifts. Any sudden adjustment in pH, carbonate hardness, light intensity, or physical substrate disturbance can trigger rapid, catastrophic Cryptocoryne melt within 24 to 72 hours of planting.
The process begins as tiny microscopic pinholes across the leaf lamina that rapidly coalesce until entire rosettes liquefy into brown, gelatinous mucilage. During this active breakdown phase (Days 1 to 3), hobbyists frequently make the critical error of excavating the plant. Following complete foliar collapse, the subterranean rhizome enters a quiescent root latency phase lasting approximately 7 days (Days 3 to 10), during which it recalibrates internal turgor pressure and anchors nascent feeder roots into the substrate. Between Days 14 and 21, compact, submersed-adapted leaves unfurl directly from the buried crown. As long as the underground rhizome remains firm, the specimen is fully viable.
Rosette Heavy Root Feeders (Echinodorus and Vallisneria)
Amazon Swords (Echinodorus bleheri, Echinodorus grisebachii) are cultivated almost exclusively emersed, featuring stiff, oval leaves with thick cuticles supported by rigid upright petioles. When undergoing the emersed to submerged transition, the plant shifts its energy toward producing narrow, strap-like, translucent foliage from the center of the basal rosette. The older emersed outer leaves turn pale yellow and dissolve over a 2 to 4 week window. Because Echinodorus species are obligate root feeders, inserting basal root tabs directly adjacent to their heavy root systems accelerates aquatic leaf formation.
Conversely, Vallisneria species are obligate submersed plants that do not possess an emersed growth form. When Vallisneria melts, the trigger is typically mechanical root crushing during planting, parameter shock from soft acidic water transitions, or chemical sensitivity to liquid glutaraldehyde additives. Crushed basal crowns cause the long, ribbon-like blades to turn transparent and slough away within days. Ensuring the pale basal crown remains positioned slightly above the substrate line prevents crown suffocation and initiates side-runner propagation within 14 days.
Fast-Growing Stem Plants (Rotala, Ludwigia, and Hygrophila)
Stem plants (such as Rotala rotundifolia, Ludwigia repens, and Hygrophila pinnatifida) display acropetal senescence during acclimation. The rounder emersed foliage along the lower two-thirds of the stem turns yellow, becomes translucent, and drops off within 3 to 5 days due to lower water-column light penetration and nutrient reallocation toward the growing apical tip.
By Day 7, the apical meristem adapts to underwater gas diffusion, sprouting narrower, vibrant leaves accompanied by adventitious water roots extending from the stem nodes. Once new aquatic terminal shoots reach 5 to 8 cm in length (typically between Days 10 and 14), cut the healthy submerged top growth, discard the bare, decomposing lower emersed stem, and replant the acclimatized cutting directly into the substrate.
Epiphytic Rhizome Flora (Anubias, Bucephalandra, and Microsorum)
Slow-growing rheophytes and epiphytes—as detailed in our Anubias nana care guide—possess tough, leathery foliage protected by dense structural cuticles. These species rarely undergo rapid, widespread leaf dissolution unless subjected to acute ammonia spikes or excessive temperatures.
Instead, mortality in epiphytic flora almost always stems from rhizome rot. Burying the horizontal creeping rhizome under fine sand or dense aqua soil cuts off interstitial water flow, creating localized rhizosphere hypoxia that allows pathogenic aquatic fungi and opportunistic bacteria to attack the plant’s core. Mount epiphytes directly onto hardscape elements like driftwood or porous stone using thread or cyanoacrylate gel to keep the rhizome exposed to circulating, oxygen-rich water. If a rhizome turns soft, black, and foul-smelling, excise the infected section 5 mm into firm, healthy green tissue using a sterile blade; replacement foliage will emerge from viable nodes within 21 to 28 days.
Preventative Acclimation Protocols for Future Plant Additions
Minimizing the severity of foliar dissolution prior to planting saves weeks of ecosystem stabilization and accelerates overall aquarium plant melt recovery. While hobbyists often look for solutions only after observing why are new aquarium plants melting and dying, implementing proactive quarantine and acclimation workflows mitigates tissue shock before botanicals ever enter the display tank.
Gradual Osmotic Drip Acclimation
Placing newly acquired potted, bunched, or tissue culture specimens into a shallow staging container and dripping display aquarium water into the basin over 30 to 45 minutes equalizes temperature, pH, GH, and total dissolved solids. This gradual adjustment prevents violent osmotic pressure swings across semi-permeable cell walls, eliminating the acute osmotic shock in planted tanks that triggers sudden vacuolar plasmolysis and early epidermal sloughing.
Rockwool Stripping and Root Sanitization
Commercial potted plants cultivated for the emersed to submerged transition arrive rooted in dense mineral rockwool saturated with terrestrial nursery fertilizers. Prior to tank placement, gently tease away 100% of the rockwool fibers under lukewarm running water using fine curved pinsettes. Leaving residual rockwool traps heavy fertilizer salts that leach uncontrolled ammonia into the substrate, while entangling nascent root tips and restricting freshwater circulation around the developing crown.
Tissue Culture Agar Gel Removal
Although in vitro tissue culture plantlets are sterile and pest-free, the nutrient-rich carbohydrate agar gel surrounding their root base presents a significant biological hazard. Every trace of culture gel must be rinsed clean in lukewarm water before division and planting. If buried beneath the substrate, residual sucrose and agar feed explosive heterotrophic blooms, stripping pore-water oxygen and creating localized rhizosphere hypoxia that rots fragile root collars within days.
Biofilter Preparation and Carbonate Hardness Buffering
Because newly introduced amphibious flora inevitably shed a fraction of their terrestrial leaves, closed aquatic systems must possess sufficient biological filtration capacity before new additions arrive. Confirm that Total Ammonia Nitrogen (TAN) and nitrite (NO2–) test at absolute zero, and verify that the system maintains a carbonate hardness (KH) buffer above 50 mg/L (CaCO3). A resilient biofilter rapidly oxidizes organic nitrogen spikes, while adequate alkalinity protects delicate tissues from biogenic decalcification during the initial photoperiod acclimation phase.
Conclusion
Understanding why are new aquarium plants melting and dying transforms an alarming visual setback into a predictable, manageable phase of planted tank maturation. Rather than signaling botanical mortality, early foliar dissolution reflects an evolutionary survival mechanism where amphibious macrophytes navigate the emersed to submerged transition by dismantling obsolete terrestrial leaves. Through cellular autophagy, plants systematically resorb mobile macronutrients from older fronds to construct thin, cuticle-free aquatic foliage engineered for submerged gas and nutrient diffusion.
Achieving a swift and resilient aquarium plant melt recovery comes down to biochemical patience and environmental discipline. By resisting the impulse to disturb dormant crowns, delaying pruning until nutrient resorption is complete, maintaining a 6-hour daily photoperiod acclimation schedule, and exporting leached organic detritus before bacterial blooms or ammonia spikes occur, aquarists can guide delicate flora through the acclimation curve and establish a thriving, vibrant planted aquascape.
Frequently Asked Questions (FAQs)
Should a melting aquarium plant be pulled out if all its leaves dissolve?
No, you should never uproot a plant merely because its foliage has dissolved. As long as the subterranean root crown, bulb, or rhizome remains firm and exhibits white, tan, or green coloration, the botanical structure remains metabolically viable and is actively storing energy to build new aquatic foliage. Excavating a leafless specimen shears off delicate, single-celled regenerating root hairs, inducing acute physical trauma and resetting the aquarium plant melt recovery timeline back to day one.
How long does aquarium plant melt recovery take?
A full aquarium plant melt recovery typically takes between 1 and 4 weeks, depending on the botanical family, lighting intensity, and nutrient stability. Fast-growing stem flora like Rotala and Hygrophila frequently sprout submerged shoots within 7 to 10 days. In contrast, specimens undergoing severe Cryptocoryne melt typically remain in a subterranean root latency phase for 10 to 14 days before unfurling new leaves between Days 14 and 21, while slow-growing epiphytic genera such as Anubias and Bucephalandra require 3 to 4 weeks or longer.
Can melting aquarium plants cause cloudy water or ammonia spikes?
Yes, decomposing plant detritus directly impacts water quality. When melted leaves lyse, they release high concentrations of Labile Dissolved Organic Carbon (LDOC) and structural plant proteins into the water column. This organic surge fuels rapid heterotrophic bacterial blooms that double every 15 to 20 minutes—creating cloudy white water—while mineralizing into toxic un-ionized ammonia (NH3) that triggers opportunistic algae outbreaks if rotting biomass is not promptly siphoned out.
Does liquid CO2 stop new aquarium plants from melting?
No, liquid carbon products cannot prevent or arrest plant melt. These liquid additives contain glutaraldehyde or related dialdehydes, which function as cellular cross-linking algaecides rather than bioavailable dissolved CO2 gas. Dosing liquid carbon onto transitioning plants damages fragile new cellular membranes and accelerates severe tissue dissolution, particularly in sensitive species such as Vallisneria and Cryptocoryne.
Why do tissue culture plants melt even though they do not have emersed leaves?
While tissue culture (in vitro) cups do not contain fully mature emersed terrestrial leaves, they are grown under 100% relative humidity with unrestricted atmospheric CO2 on a nutrient-rich agar gel matrix. Submerging these micro-cuttings into an aquarium still requires metabolic acclimation to aquatic carbon diffusion and parameter differences, causing minor osmotic shock in planted tanks. Furthermore, failing to wash off 100% of the nutrient agar gel fuels anaerobic bacterial rot and localized ammonia burn directly at the substrate line.
